elocation-id: elocation-id: e4264
Pigeon peas, Cajanus cajan (L.) Millsp, are a legume of great nutritional importance due to their nutritional quality and ability to adapt to adverse conditions. The study was conducted in 2024 at the College of Postgraduates, Montecillo, Texcoco, State of Mexico, with the aim of evaluating the effects of citrulline and humic acids, applied as treatments, on germination, vigor and biomass accumulation in Cajanus cajan (L.) Millsp., under greenhouse conditions. Four treatments were evaluated: control without treatment, citrulline (1 g L-1), humic acids (1 ml L-1), and the combination of citrulline + humic acids, using a completely randomized design. The germination variables evaluated, such as the number of seeds germinated, germination percentage, mean germination time, mean germination rate, germination uncertainty index, and germination synchrony index, did not show significant differences between treatments, indicating that the seed had high viability. At 120 days after sowing, significant differences were observed in leaf dry matter accumulation, with greater values in treatments with citrulline and citrulline + humic acids. The slenderness index did not differ between treatments; however, the plant vigor index was higher in the combination of citrulline + humic acids compared to the control. The results indicate that, although pre-germination treatments did not affect germination, citrulline promoted the accumulation of leaf biomass and, when combined with humic acids, promoted greater plant vigor.
biostimulant, feasibility, fodder, germplasm.
Pigeon peas, Cajanus cajan (L.) Millsp., are a shrub legume with diverse uses in agricultural and food systems, valued for its tolerance to semi-arid conditions and its potential as a multipurpose crop (grain, fodder and green manure), with biomass production of up to 24 t ha-1. In the literature, Cajanus cajan (L.) Millsp. is described as a relevant agronomic option for marginal areas due to its edaphoclimatic adaptation and its protein contribution of up to 22% in human and animal diets (Atuna et al., 2023; Bopape et al., 2023).
In addition, this crop participates in the biological fixation of nitrogen, with rates of 80 to 230 kg ha-1, which improves soil fertility and contributes to the sustainability of cultivation systems by reducing the use of synthetic nitrogen fertilizers (Bopape et al., 2023).
Germination and seedling vigor are critical factors in the establishment and final yield of crops; the speed of implantation, uniformity of emergence, and the ability to tolerate abiotic stress in the initial stage directly influence productivity (Reed et al., 2022). In many legumes, dormancy due to impermeability of the seed testa limits the imbibition process, with the consequent decrease in the speed and synchrony of germination.
In some plant species, the structure and composition of the seed integument cause impermeability; nevertheless, there are field and laboratory methods that accelerate emergence and germination, including mechanical and chemical scarification, heat or osmotic treatments, and the use of biostimulants (Wen et al., 2024).
Among biostimulants, citrulline has been described as a non-protein amino acid involved in nitrogen metabolism, osmotic functions and redox regulation, and it also participates in repair pathways and in nitrogen transport to growing tissues in Cucurbitaceae (Joshi and Fernie, 2017; Song et al., 2020).
Physiological and transport studies detected the presence of citrulline in sap and young tissues, suggesting its role in mobilizing nitrogenous compounds during germination and early growth in Juglans regia L. (Mapelli et al., 2001; Song et al., 2020).
On the other hand, humic acids obtained from organic matter have promoting effects on root physiology, nutrient absorption, and enzymatic activity related to the antioxidant protection of seeds and seedlings. Recent experimental studies show increased germination rates and seedling vigor after applications of humic acids across different crops and stress conditions (Basahi, 2021; Yang et al., 2023).
Although there is evidence supporting the use of citrulline and humic acids as establishment promoters in various species, such as cucurbits and grasses, the number of studies focused on legumes, particularly Cajanus cajan (L.) Millsp., remains limited.
Based on the above, this study aimed to evaluate the effects of applying citrulline and a commercial humic acid on the parameters of germination, emergence uniformity, and initial development of Cajanus cajan (L.) Millsp. seedlings under greenhouse conditions.
The research was conducted in a greenhouse of the Center for Training and Technological Innovation (CCIT, by its Spanish initialism) of the College of Postgraduates-Montecillo Campus, located in Montecillo, Texcoco, State of Mexico.
The present study used seeds harvested five months before the research was established, collected from plants previously established on the Campus, which were subjected to different pre-germination treatments.
Pre-germination treatments were evaluated: T1= seed without pretreatment; C treatment= 1 h of immersion in 1 L of water, added with 1 g of citrulline powder (L-citrulline, Evolution®); HA treatment= 1 h of immersion in 1 L of water, added with 1 ml of Agrobeta® humic acids; and C+HA treatment= 1 h of immersion in 1 L of water, added with 1 g of citrulline + 1 ml of humic acids.
After treating the seeds, sowing was carried out. To this end, 200-300-gauge nursery bags (27 cm x 27 cm) were used and filled with soil from the ‘Predio Nuevo’ plot (sandy clay loam texture, pH of 7.9 and an organic matter content of 2%) on the same Montecillo Campus.
A seed was placed in each bag at a depth of two centimeters and 25 bags were assigned to each treatment. Finally, saturation irrigation was applied to promote germination and repeated every third day until the conclusion of the work.
During the evaluation period, the temperature inside the greenhouse was recorded using an RC-5+ data logger (Elitech Technologies, Milpitas, CA, USA).
Seedling emergence was monitored for 30 days after sowing, in the morning between 8 and 9 am, throughout the assessment. The above was done in order to calculate the speed of emergence (Maguire, 1962), number of germinated seeds (ngs), percentage of germination (pg), mean germination time (mgt), mean germination rate (mgr), germination uncertainty index (unc), and germination synchrony index (syn) on the platform (Kim et al., 1987; Ranal and Santana, 2006; Martínez et al., 2010; ISTA, 2018).
Seedlings were considered to have emerged once the plumule hook was observed at the soil surface and the process of photosynthetic autotrophism initiated (Forcella et al., 2000).
On day 120 after sowing (DAS), a destructive sampling was carried out, in which five plants were randomly selected per treatment. In this sampling, plant height (cm), number of trifoliate leaves and diameter of the root neck (mm) were measured.
This information was used to calculate the slenderness index (SI) employing the following equation:
In addition, the plant vigor index (PVI) was determined with the equation proposed by Kim et al. (1987):
On the other hand, the dry matter of the morphological components (roots, stems, and leaves) was also obtained. Dry matter was obtained by recording the fresh weight (g) of each component on a KMT® Style analytical balance, with a margin of error of ±0.1 g and ±0.01 g.
The samples were placed in paper bags identified by the morphological component and dried in a forced-air drying oven at 55 °C for 72 h until a constant weight was reached; thereafter, only the difference between the fresh and dry weights was calculated.
The analysis of variance of the data considered a completely randomized experimental design with five replications per treatment. The comparison of means was made using Tukey’s test (p< 0.05). Statistical analyses were performed with SigmaPlot 15 (Systat Software, San Jose, California, USA).
The results (Table 1) indicate that none of the germinative variables presented significant differences (p> 0.05) between treatments.
The lack of effect of pre-germination treatments on germination could be explained by the high initial viability of the seed, which was used five months after harvest and because the experimental conditions favored germination, thereby narrowing the response window to biostimulants applied to the seed, a phenomenon that is similar to that observed in other studies with germplasm of high physiological quality in corn and sorghum (Nicchio et al., 2013; Vendruscolo et al., 2014; Rodrigues et al., 2017).
In the analysis of growth and biomass accumulation at 120 days after sowing (Table 2), only the proportion of dry matter in leaves (DM-l) showed significant differences among treatments (p= 0.002). Treatments with citrulline and the combination of citrulline + humic acids showed greater accumulation of leaf mass compared to the control. This suggests a physiological effect of citrulline on the partitioning of biomass towards leaves in Cajanus cajan (L.) Millsp.
[i] Plant height (H, cm); number of leaves (NL); root neck diameter (SD, mm); dry matter in leaves (DM-l, %); dry matter in stem (DM-s, %); dry matter in root (DM-r, %) in Cajanus cajan (L.) Millsp. plants obtained from seeds subjected to different pre-germination treatments 120 days after sowing. The values presented are the mean of five observations and their standard error.
Citrulline acts as a compatible osmolyte, a chelator of reactive oxygen species and a modulator of amino acid metabolism and other nitrogen-related pathways; these mechanisms can increase biomass under limited nitrogen conditions (Joshi and Fernie, 2017; Song et al., 2020).
In addition, recent research shows that citrulline priming and exogenous citrulline application improve growth parameters and tolerance to abiotic stress (Song et al., 2020; Farooq et al., 2025). Nonetheless, under non-stressful conditions, the effect on germination is usually small (Song et al., 2020; Farooq et al., 2025), which is consistent with the results observed in this research.
Regarding the effects of humic acid, its effectiveness has been shown to depend on the source, molecular structure, dose and crop conditions. In addition, positive effects on growth, biomass, root architecture and nutrient use efficiency tend to manifest in seedling development rather than in the germination of seeds with high viability (Nunes et al., 2019; Nardi et al., 2021; Yang et al., 2023; Vitti et al., 2024).
Recent work shows that certain humic acid fractions regulate plasma membrane H+-ATPase activity, Ca2+ signaling, and TOR kinase activation (target of rapamycin), all of which stimulate initial root growth (Canellas et al., 2022; Nabi et al., 2025; Santos et al., 2025).
Such mechanisms explain why, even without an effect on germination, the presence of humic acids can indirectly increase seedling development and biomass accumulation observed in some of the treatments used in the present study (Nardi et al., 2021; Yang et al., 2023).
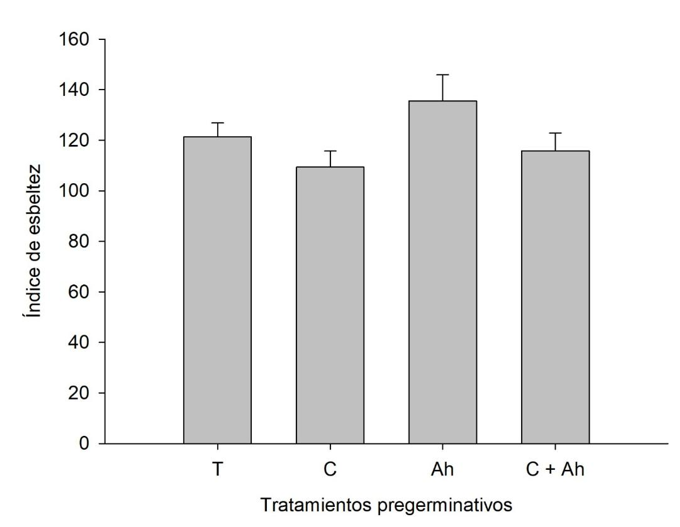
The slenderness index showed no significant differences (p> 0.05) among seedlings obtained from seeds subjected to different pre-germination treatments (Figure 1). This indicates that the root neck diameter/height ratio remained stable in all treatments evaluated.
In contrast, the plant vigor index showed significant differences (p= 0.018). Plants originating from seeds treated with the C + HA combination exhibited superior vigor compared with the control (Figure 2).
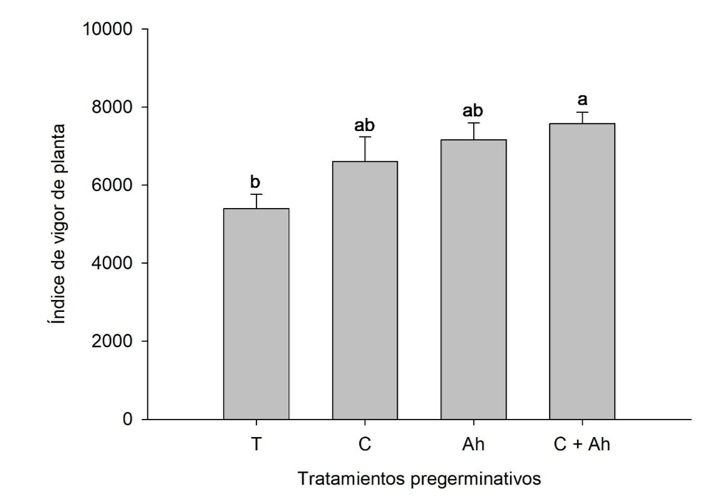
This result suggests a synergistic interaction between citrulline and humic acids that favors vigor attributes in the medium term, possibly through an improvement in antioxidant protection (by citrulline) and stimulation of nutrient acquisition and root remodeling (by humic acids).
Recent observations support the hypothesis of synergy between biostimulant amino acids and humic substances, as they enhance plant response under stress conditions and improve nutritional efficiency (Canellas et al., 2022; Nabi et al., 2025).
The application of citrulline favored the accumulation of leaf dry matter, and humic acids are more relevant during the seedling development phase and in root remodeling during germination; however, when combined with citrulline, they showed positive effects on plant vigor.
This offers the possibility of applying citrulline and humic acids as a biostimulation strategy, with a greater probability of observing positive effects when the seed has low viability or when seedlings are under stress or nutritional limitations.
Atuna, R. A.; Mensah, M. A. S.; Koomson, G.; Akabanda, F.; Dorvlo, S. Y. and Amagloh, F. K. 2023. Physico-functional and nutritional characteristics of germinated pigeon pea (Cajanus cajan) flour as a functional food ingredient. Reino Unido. Scientific Reports. 13(1):16627. https://doi.org/10.1038/s41598-023-43607-8.
Canellas, L. P.; Canellas, N. O. A.; da Silva, R. M.; Spaccini, R.; Mota, G. P. and Olivares, F. L. 2022. Biostimulants using humic substances and plant-growth-promoting bacteria: effects on cassava Manihot esculentus and okra Abelmoschus esculentus yield. Suiza. Agronomy. 13(1):80- https://doi.org/10.3390/agronomy13010080.
Farooq, U.; Ashraf, M. A.; Iqbal, M. and Rasheed, R. 2025. Effect of citrulline seed priming on growth, photosynthesis, redox equilibrium, secondary metabolic enzymes, metal sequestration and nutrient acquisition in sunflower Helianthus annuus L. under chromium toxicity. Suiza. BioMetals. 38(6):1991-2018. https://www.semanticscholar.org/paper/Effect-of-citrulline-seed-priming-on growth%2C-.
Nunes, R. O.; Domiciano, G. A.; Alves, W. S.; Melo, A. C. A.; Nogueira, F. C. S.; Canellas, L. P.; Olivares, F. L.; Zingali, R. B. and Soares, M. R. 2019. Evaluation of the effects of humic acids on maize root architecture by label-free proteomics analysis. Reino Unido. Scientific Reports. 9(1):12019. https://doi.org/10.1038/s41598-019-48509-2.
Santos, M. P.; Zupunski, M.; Monda, H.; Gralian, J.; James, A.; Grossmann, G.; Lamar, R. T. and Zandonadi, D. B. 2025. Humic acids modify root architecture in Arabidopsis through H+-ATPase-dependent target of rapamycin activation in concert with a2+ and ROS signaling. Italia. Chemical and Biological Technologies in Agriculture. 12(1):1-15. https://link.springer.com/article/10.1186/s40538-025-00764-4.
Torres, A.; Cova, A. y Varela, D. 2008. Efecto del proceso de germinación de granos de Cajanus cajan en la composición nutricional, ácidos grasos, antioxidantes y bioaccesibilidad. Chile. Revista Chilena de Nutrición. 45(5):323-332. https://www.scielo.cl/scielo.php?script=sci-arttext&pid=S0717-75182018000500323.
Vitti, A.; Coviello, L.; Nuzzaci, M.; Vinci, G.; Deligiannakis, Y.; Giannakopoulos, E.; Ronga, D.; Piccolo, A.; Scopa, A. and Drosos, M. 2024. Biostimulation of humic acids on Lepidium sativum L. regulated by their content of stable phenolic O⋅ radicals. Suiza. Chemical and Biological Technologies in Agriculture. 11(2):92. https://link.springer.com/article/10.1186/s40538-024-00613-w.